Marine Reptiles of the Dinosaur Age: Mosasaurs, Plesiosaurs, and Ichthyosaurs
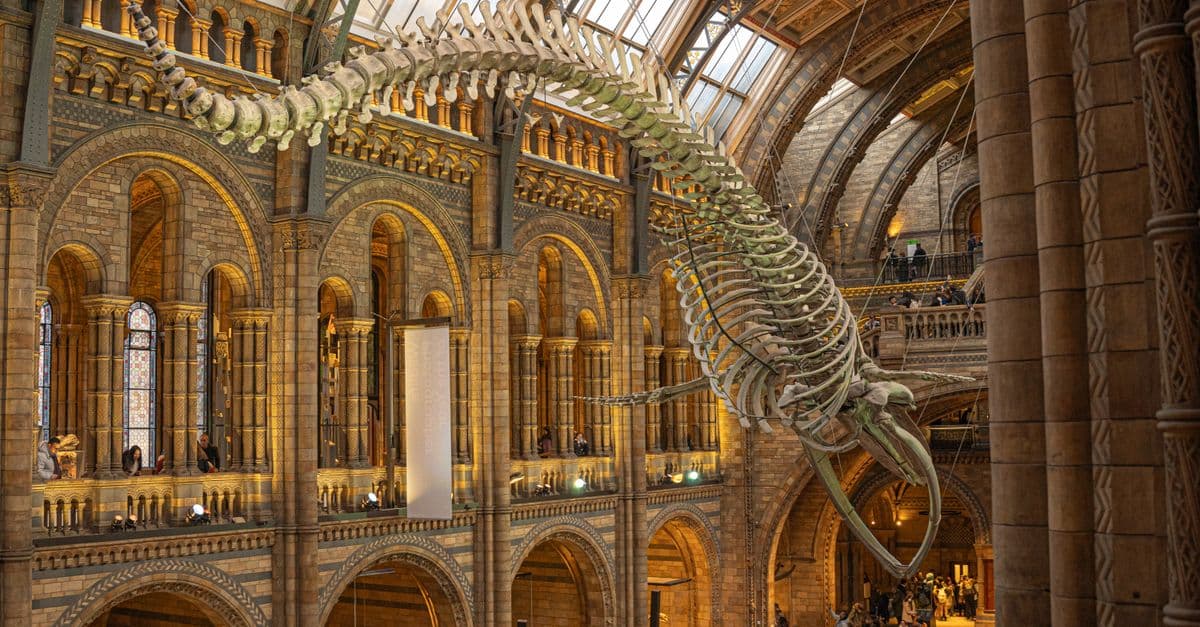
Photo: Sebastian Dziomba / Pexels
The Mesozoic oceans were not passive background to the dinosaur story on land. They were contested, productive, and ruled by predators that evolution had pulled back from land into water — a transition that happened not once but at least three separate times, in three separate reptile lineages. Mosasaurs, plesiosaurs, and ichthyosaurs each solved the problem of aquatic predation differently, each reached sizes that dwarf any modern marine predator except the sperm whale, and each went extinct 66 million years ago in the same event that ended the non-avian dinosaurs. None of them were dinosaurs. All of them were extraordinary.
What These Animals Were — And Were Not
The most persistent public misconception is that mosasaurs, plesiosaurs, and ichthyosaurs were marine dinosaurs. They were not. They were not dinosaurs at all.
Dinosauria is a specific clade defined by a set of anatomical characters — particularly a fully erect posture with the femur fitting into a fully open hip socket, specific features of the ankle and ankle musculature, and several skull characteristics. None of the marine reptile groups share these diagnostic features. They belong to separate evolutionary lineages within the broader group of reptiles.
Ichthyosauria — a clade of fully aquatic marine reptiles that flourished from the Triassic through the mid-Cretaceous; likely descended from a terrestrial diapsid ancestor that returned to the sea, though the exact ancestor remains uncertain.
Plesiosauria — a clade of Mesozoic marine reptiles divided into long-necked plesiosaurs (plesiosaurs) and large-headed short-necked forms (pliosaurs), all using four large paddle-like limbs for propulsion.
Mosasauridae — a family of large marine lizards within the squamate lineage (the group containing modern lizards and snakes), which evolved in the Late Cretaceous from monitor lizard-like ancestors.
Each of these groups has a different relationship to other modern reptiles. Ichthyosaurs are diapsid reptiles of uncertain exact affinity. Plesiosaurs belong to Sauropterygia, a broader marine reptile clade. Mosasaurs are squamates — their closest living relatives are Komodo dragons and snakes. Living alongside dinosaurs does not make an animal a dinosaur, any more than living alongside humans makes a dolphin a primate.
Source: Motani, R., Annual Review of Earth and Planetary Sciences (2009) — Comprehensive review of ichthyosaur evolution and convergence with modern cetaceans.
Source: Palci, A. et al., Zoological Journal of the Linnean Society (2013) — Phylogenetic analysis of mosasaur relationships within Squamata, confirming their close affinity with varanid lizards.
Ichthyosaurs: The Dolphins That Came First
Ichthyosaurs are the most remarkable example of convergent evolution in the vertebrate fossil record. Convergent evolution is the process by which unrelated lineages independently evolve similar anatomical solutions to the same environmental challenge — like the dolphin body plan appearing in both mammals (dolphins) and reptiles (ichthyosaurs) separated by over 200 million years.
Convergent evolution — the independent evolution of similar anatomical features in distantly related lineages, driven by similar selective pressures in similar environments; ichthyosaurs and dolphins are the textbook example.
A fully developed ichthyosaur like Ichthyosaurus communis from the Jurassic of England is almost indistinguishable in body outline from a modern dolphin: streamlined torpedo body, tall dorsal fin, crescent-shaped tail fin (with the tail driving the lower lobe, unlike fish where the backbone extends into the upper lobe — an important anatomical difference), long snout packed with conical teeth, and large eyes. It had flippers instead of legs, breathed air via nostrils at the top of the snout, and almost certainly gave birth to live young rather than laying eggs — a rare trait for a reptile, and one we know with certainty because fossils of Stenopterygius from Germany preserve individuals in the act of giving birth, with young exiting tail-first (as modern cetaceans do, to prevent drowning before birth is complete).
The ichthyosaur eye is worth special attention. Temnodontosaurus platyodon, a large Early Jurassic ichthyosaur, had an eye with a sclerotic ring diameter of approximately 25 cm — potentially the largest eye of any vertebrate known. Large eyes in deep-diving marine animals are associated with vision in low-light, deep-water environments. Modern sperm whales, which dive to 2,000 m in darkness, have eyes roughly 17 cm across. Temnodontosaurus may have been diving to comparable depths in Jurassic seas.
| Ichthyosaur | Length | Period | Notable Feature |
|---|---|---|---|
| Mixosaurus | ~1 m | Middle Triassic | Transitional — still had a fish-like tail |
| Ichthyosaurus | ~2 m | Early Jurassic | Dolphin-like; common in English deposits |
| Temnodontosaurus | ~9 m | Early Jurassic | Largest eye of any known vertebrate |
| Shastasaurus | ~21 m | Late Triassic | Possibly the largest ichthyosaur; toothless adult |
| Ophthalmosaurus | ~6 m | Late Jurassic | Enormous eyes; deep-diver morphology |
Ichthyosaurs are known from the Triassic through the mid-Cretaceous. They diversified explosively in the Triassic — transitional forms like Mixosaurus still show some fish-like tail proportions, while fully derived Jurassic forms had achieved the complete dolphin-equivalent body plan. They declined in diversity through the Cretaceous, with the last ichthyosaurs disappearing approximately 90 Ma — roughly 24 million years before the end-Cretaceous extinction — apparently outcompeted by mosasaurs and sharks in many ecological niches.
Source: Motani, R. et al., Science (1998) — Description of Utatsusaurus and early ichthyosaur evolution, tracing the transition from terrestrial ancestor to fully aquatic form.
Source: Johnson, R., Journal of Vertebrate Paleontology (1977) — Analysis of Temnodontosaurus eye structure, establishing it as one of the largest vertebrate eyes known from the fossil record.
Plesiosaurs: Four Paddles, Two Strategies
Plesiosaurs present a different evolutionary strategy from ichthyosaurs. Where ichthyosaurs converged on the dolphin body plan — single-axis tail propulsion — plesiosaurs evolved a completely novel solution: four large, wing-like flippers generating thrust simultaneously, like an underwater bird using all four limbs as wings.
This mode of locomotion — underwater flight — is shared with modern sea turtles, penguins, and sea lions (though each uses a slightly different limb configuration). Biomechanical analysis of plesiosaur forelimb anatomy suggests the forelimbs provided most of the propulsive force, with the hindlimbs contributing stability and maneuverability. The four-flipper arrangement allowed exceptional agility — the ability to rotate tightly and reverse direction in ways that tail-propelled animals cannot easily match.
Within Plesiosauria, two radically different body plans evolved:
Plesiosaurs (long-necked forms): Families like Elasmosauridae had extraordinarily long necks with up to 76 vertebrae (for comparison, a giraffe has 7, all mammals do). Elasmosaurus platyurus had a neck roughly 7 m long on a total body length of ~14 m. The function of the long neck has been debated for over a century. Likely uses include stalking fish schools from below (approaching slowly with the small head before striking), reaching into rocky crevices, or ambush predation in shallow coastal environments. The neck was not flexible enough to arch dramatically over the back — a persistent popular image that the anatomy does not support.
Pliosaurs (short-necked forms): Pliosauridae evolved in the opposite direction — short, massive necks; huge, powerful skulls; and enormous bite force. Predator X (formally Pliosaurus funkei), described from Svalbard in 2012, had a skull estimated at 2–3 m long with a bite force estimated at 15 tonnes — greater than any other known animal. It reached approximately 10–13 m in total length. Pliosaurs were the apex pelagic predators of the Jurassic oceans, filling the ecological role occupied by modern orcas and great white sharks combined.
Source: Knutsen, E.M. et al., Norwegian Journal of Geology (2012) — Description of Pliosaurus funkei from Svalbard, with bite force estimates placing it among the most powerful predators in Earth's history.
Source: O'Keefe, F.R., Paleobiology (2001) — Quantitative analysis of plesiosaur body plan evolution, demonstrating the polarity of the long-neck/short-neck split within Plesiosauria.
The Plesiosaurus Neck Debate: How Did It Actually Move?
The long neck of plesiosaurs has generated a persistent misunderstanding — the idea that they could rear the neck high above the water surface like a swan, or arch it dramatically in a curve. This image shaped the "Loch Ness Monster" mythology and countless outdated book illustrations.
Anatomical analysis of plesiosaur neck vertebrae shows they were designed primarily for lateral (side-to-side) flexibility, with limited dorsal (upward) bending. The neck could sweep horizontally through a wide arc — useful for ambush predation — but could not easily curve vertically into the high-arching poses of popular imagination. It moved more like a horizontal boom than a vertical periscope.
The long neck may also have functioned in sexual selection — longer-necked individuals being preferred mates — or in intraspecific competition. Modern giraffes' necks are partially explained by male competition (necking behavior), not purely by foraging reach. Plesiosaur necks may have followed a similar mixed-selection pathway.
Source: Zammit, M. et al., Journal of Vertebrate Paleontology (2008) — Range of motion analysis in plesiosaur cervical vertebrae, demonstrating primarily lateral flexibility and limited dorsal extension.
Mosasaurs: The Last and Largest Mesozoic Ocean Predators
Mosasaurs are the newest arrival among Mesozoic marine reptiles — they appear in the fossil record only in the Late Cretaceous, roughly 98 Ma, and went extinct 66 Ma at the Cretaceous-Paleogene boundary. In their 32-million-year existence, they became the dominant ocean predators of the Cretaceous and reached extraordinary sizes.
Mosasaurs are lizards — or more precisely, they are derived members of Squamata, the order containing modern lizards and snakes. Their closest living relatives are the varanid lizards (monitors, including the Komodo dragon), though the squamate lineage leading to mosasaurs branched off from the lineage leading to modern varanids well before mosasaurs became marine.
The transition from terrestrial lizard to fully marine predator is documented in early mosasaur forms like Dallasaurus turneri and Russellosaurus coheni, which retain some terrestrial-capable limb anatomy. Later mosasaurs show progressive transformation of the limbs into flippers, development of a tail fin, and deepening of the body for aquatic locomotion. The tail fin of advanced mosasaurs was a hypocercal (downward-bent) tail — the backbone bent downward into the lower tail lobe, while the upper lobe was supported by soft tissue. This is opposite to the tail structure of sharks (where the backbone extends into the upper lobe) and represents another independent invention of the aquatic tail fin.
| Mosasaur | Length | Location | Notes |
|---|---|---|---|
| Dallasaurus | ~1 m | Texas, USA | Transitional; earliest known mosasaur |
| Platecarpus | ~7 m | North America | Medium-bodied; well-preserved soft tissue |
| Tylosaurus | ~12–14 m | North America / Europe | Dominant apex predator; ate other mosasaurs |
| Mosasaurus hoffmannii | ~17 m | Europe / Africa | Largest known mosasaur; enormous skull |
| Hainosaurus | ~15 m | Europe | Rival to Mosasaurus in size |
Mosasaurus hoffmannii is the type species of the group, first described in 1822 from a skull found in the Saint-Pieter mountain near Maastricht, Netherlands — making it one of the first prehistoric reptiles to be formally described scientifically, predating the word "dinosaur" by two decades.
Mosasaurs were generalist apex predators with diverse diets documented by fossilized stomach contents: fish, cephalopods (ammonites), sea turtles, plesiosaurs, sharks, and other mosasaurs. Tylosaurus proriger specimens from Kansas preserving gut contents have been found containing mosasaur and plesiosaur bones — these were animals eating other large marine reptiles.
Source: Caldwell, M.W. & Lee, M.S.Y., Proceedings of the Royal Society B (1997) — Analysis of mosasaur origins within Squamata, documenting their close relationship to varanid lizards and the transition from terrestrial to marine lifestyle.
Source: Everhart, M.J., Oceans of Kansas (Indiana University Press, 2005) — Documentation of mosasaur diet from preserved gut contents in Cretaceous Western Interior Seaway specimens.
Convergent Evolution: The Ocean Keeps Reinventing the Same Shapes
The story of Mesozoic marine reptiles is, at a deeper level, a story about how predictable evolution can be when environments impose strong, consistent selective pressures.
The ocean selects for streamlined bodies (drag reduction), large size (thermal inertia and predator dominance), live birth (no returning to land to lay eggs), large eyes (vision in dim water), and specific tooth shapes (conical teeth for fish; crushing teeth for shellfish). Ichthyosaurs, plesiosaurs, and mosasaurs each converged on subsets of these solutions independently. Ichthyosaurs converged most completely on the dolphin body plan. Mosasaurs converged on an elongated, serpentine plan resembling modern sea snakes at vast scale. Plesiosaurs invented a unique locomotor strategy that no other vertebrate lineage has replicated.
Modern dolphins, which returned to the sea from land mammals about 50 million years ago, independently reinvented the same streamlined body plan that ichthyosaurs had perfected 200 million years earlier. This is not coincidence — it is the same environment producing the same solutions through the same physical laws.
The implication is both humbling and clarifying: evolution is not infinite in its creativity. Physical constraints channel it into predictable outcomes. Given an ocean, given an amniote ancestor on land, given enough time, you will get something that looks like a dolphin.
Source: Losos, J.B., Improbable Destinies: Fate, Chance, and the Future of Evolution (Riverhead Books, 2017) — Accessible treatment of convergent evolution, with extensive discussion of marine reptile examples alongside modern cases.
What People Get Wrong About Mesozoic Marine Reptiles
The first error is the dinosaur misclassification, addressed above. The second is imagining these animals as slow, cold-blooded sea serpents — essentially big crocodilians in the open ocean.
Evidence from bone histology (growth ring analysis), stable isotope chemistry in teeth, and body plan analysis all converge on the conclusion that at least ichthyosaurs and mosasaurs were endothermic (warm-blooded) or near-endothermic. A 2020 study of ichthyosaur bone and scale chemistry found isotopic signatures indicating they maintained body temperatures significantly above the surrounding water — comparable to modern tuna and lamnid sharks (which are also warm-bodied but not technically endothermic). For animals the size of Tylosaurus, warm-bloodedness would have been nearly inevitable through thermal inertia alone, even without active thermogenesis.
The third error is the "Loch Ness Monster might be a plesiosaur" idea. Plesiosaurs were air-breathers that would need to surface regularly. Any large, extant plesiosaur population in Loch Ness would leave unambiguous evidence — regular sightings of surfacing animals, bodies, bones, DNA in the water. Environmental DNA surveys of Loch Ness water have detected no unusual species. The Loch Ness Monster does not exist, and no plesiosaur survived the Cretaceous extinction. These are two separate facts that independently exclude the possibility.
Source: Bernard, A. et al., Science (2010) — Oxygen isotope analysis of ichthyosaur teeth indicating elevated body temperatures relative to ambient seawater, consistent with partial or full endothermy.
The Takeaway
Three independent lineages of land reptiles looked at the Mesozoic ocean and went back in. Each solved the problem of large-scale marine predation differently: ichthyosaurs built a dolphin, plesiosaurs built an underwater bird, and mosasaurs built a sea serpent with a lizard's skull. All three reached sizes that no marine predator has matched since. All three went extinct 66 million years ago — their slot in the ocean eventually filled by the true cetaceans, who ran the same evolutionary experiment 50 million years later and arrived at many of the same answers. The ocean, it turns out, has a preferred shape for large, air-breathing predators. It just needs something from land to start with.
Frequently Asked Questions
Q: Were mosasaurs, plesiosaurs, and ichthyosaurs dinosaurs?
A: No. None of them were dinosaurs. All three groups were reptiles that lived during the Mesozoic Era alongside dinosaurs, but they belonged to separate evolutionary lineages. Ichthyosaurs were diapsid reptiles of uncertain affinity, plesiosaurs were sauropterygian reptiles, and mosasaurs were squamates (lizards), most closely related to modern varanid lizards like the Komodo dragon.
Q: How large did mosasaurs get?
A: The largest known mosasaur, Mosasaurus hoffmannii, reached approximately 17 m (56 ft) in length — comparable to a large sperm whale in length, though far lighter. Tylosaurus proriger and Hainosaurus bernardi were close rivals at 12–15 m. For comparison, the largest modern predatory fish, the great white shark, reaches about 6 m.
Q: Could plesiosaurs lift their necks high above the water?
A: No, not dramatically. Analysis of plesiosaur neck vertebrae shows the neck was primarily flexible laterally (side-to-side) rather than vertically. The high-arching, swan-like neck posture seen in older illustrations and popularized by Loch Ness Monster imagery is anatomically unsupported. The neck swept horizontally, functioning more like an ambush tool sweeping through fish schools than a periscope.
Q: Did ichthyosaurs give birth to live young?
A: Yes — this is confirmed by fossils, not inference. Multiple specimens of Stenopterygius from the Holzmaden quarries of Germany preserve ichthyosaurs in the act of giving birth, with young in the birth canal or partially emerged. Young exited tail-first, as in modern cetaceans, preventing the young from drowning before the head fully emerges.
Q: What ate mosasaurs?
A: Larger mosasaurs ate smaller ones. Tylosaurus proriger specimens preserve the bones of other mosasaurs in their stomach contents. Large mosasaurs were likely the apex predators of the late Cretaceous open ocean with no consistent predators. Sharks coexisted but would have been prey rather than predators for large mosasaur species.
Q: Why did none of these groups survive the Cretaceous extinction?
A: The Cretaceous-Paleogene extinction (66 Ma) eliminated all non-avian marine reptiles. The exact mechanism involved the Chicxulub impact's collapse of marine food webs — the plankton and small fish that underpinned the entire oceanic food chain died off in massive numbers following the impact winter. Large apex predators, which required sustained prey availability, were among the most vulnerable. Unlike birds and small mammals on land, no marine reptile lineage survived through the ecological collapse.
Source: Twitchett, R.J., Palaeogeography, Palaeoclimatology, Palaeoecology (2006) — Analysis of food web collapse during mass extinction events, explaining the disproportionate vulnerability of large apex predators.
Source: Friedman, M., Proceedings of the Royal Society B (2012) — Comparison of ichthyosaur and dolphin body plan convergence, quantifying the degree of morphological similarity between the two independent solutions to aquatic predation.
Read next:
Follow new articles
Add SciHub101 to your feed reader to see new science and technology stories.
About the Author
SciHub101 is an independent science and technology publication founded and edited by Buğra Sözeri, a software engineer and app developer based in Türkiye. AI tools assist with drafting and research. Source documentation in the existing archive is uneven, and articles are being reviewed and corrected. The Editorial Team byline identifies editorial responsibility; it does not certify specialist or independent human review. Where we compare products, anything built by our own team is labelled as such — see the editorial guidelines and About page for how corrections and disclosures work.
Related Articles
Pterosaurs: The Flying Reptiles That Were Not Dinosaurs
Pterosaurs were the first vertebrates to achieve powered flight, doing so roughly 50 million years before birds and 80 million years before bats. At their largest — Quetzalcoatlus northropi, with a wingspan matching a small aircraft — they were the heaviest flying animals in Earth's history. Yet despite sharing the Mesozoic with dinosaurs and appearing in every dinosaur documentary, pterosaurs were not dinosaurs. They were something altogether different.
Spinosaurus: The Aquatic Dinosaur Bigger Than T. Rex
For most of the 20th century, Spinosaurus was a mystery — a massive sail-backed predator known only from destroyed World War II specimens and a handful of fragments. Then a series of discoveries between 2014 and 2020 transformed it into one of the most scientifically debated dinosaurs alive, and the only known dinosaur adapted for aquatic, tail-propelled swimming. It was also longer than Tyrannosaurus rex by several meters — and the controversy over what exactly it was is far from settled.
The Three Periods of Dinosaurs: Triassic, Jurassic, and Cretaceous
Dinosaurs did not exist in a single monolithic era. They ruled Earth across three distinct geological periods spanning 165 million years — longer than the time separating us from the last non-avian dinosaur. Each period had its own continents, climates, ecosystems, and dominant species. Understanding what changed across the Triassic, Jurassic, and Cretaceous is the key to understanding why dinosaurs became what they became.
Triceratops and the Horned Dinosaurs: Frills, Horns, and the Fossil Evidence
Ceratopsians — the horned and frilled dinosaurs — are among the most distinctive animals in the fossil record, and among the most misunderstood. Triceratops's frill was not armor. Its horns may have been used for display as much as combat. Torosaurus may or may not be a different animal from Triceratops — the debate is genuinely unresolved. And ceratopsian herds, though often depicted as vast migratory columns, are supported by specific but limited fossil evidence. Here is what the bones actually show.
Velociraptor: The Real Science Behind the Jurassic Park Icon
The Velociraptor in Jurassic Park stands 1.8 meters tall, hunts in coordinated packs, and opens doors. The actual animal was the size of a turkey, covered in feathers, and probably hunted alone. Almost nothing about cinema's most famous raptor matches the fossil record — yet the real animal is, in its own way, more interesting than the fiction.
Tyrannosaurus Rex: The Science Behind the World's Most Studied Dinosaur
T. rex is not just a cultural icon — it is the most scientifically studied non-avian dinosaur in history, with over 50 reasonably complete specimens and a research record spanning more than a century. What emerges from that scrutiny is more complex and more surprising than the movie monster: an animal with the most powerful bite force ever measured in a land animal, better depth perception than a hawk, and a growth strategy that turned a 50-kg juvenile into a 9-tonne adult in roughly 20 years.